Feature Review
Effects of Grafting on Growth and Yield of Eggplant 

2 Zhejiang Agronomist College, Hangzhou, 310021, Zhejiang, China
 Author Correspondence author
Genomics and Applied Biology, 2026, Vol. 17, No. 5
Received: 30 Aug., 2026 Accepted: 08 Oct., 2026 Published: 22 Oct., 2026
Eggplant (Solanum melongena L.) is an economically important vegetable crop widely cultivated worldwide, but its productivity is often constrained by soil-borne diseases, continuous cropping problems, and environmental stresses. Grafting has emerged as an effective and sustainable horticultural technique to enhance plant growth, improve stress tolerance, and maintain stable yield under intensive production systems. This review summarizes the effects of grafting on eggplant growth and yield formation, with emphasis on the physiological mechanisms and practical applications of different grafting strategies. The influence of grafting on vegetative growth, including plant morphology, root system development, photosynthetic performance, and biomass accumulation, is discussed in detail. Grafted eggplants generally exhibit stronger root activity, improved nutrient uptake capacity, and enhanced resource utilization efficiency due to the functional advantages of selected rootstocks. In addition, grafting contributes to yield improvement by promoting flowering, fruit setting, fruit development, and maintaining favorable fruit quality characteristics. The role of grafting in enhancing resistance against soil-borne pathogens and abiotic stresses, including drought, salinity, and temperature fluctuations, is also highlighted. A case study of grafted eggplant production under protected cultivation demonstrates that appropriate rootstock selection and integrated management practices can significantly improve plant growth performance, yield stability, and production sustainability. Despite these advantages, further research is required to optimize rootstock-scion combinations, clarify graft-induced physiological and molecular regulation mechanisms, and integrate grafting technology with precision agriculture systems. Overall, grafting represents a valuable approach for sustainable eggplant production by improving plant adaptability, productivity, and resilience under diverse cultivation environments.
1 Introduction
Eggplant (Solanum melongena L.) is one of the most important solanaceous vegetables grown worldwide and has substantial nutritional, economic, and agronomic value in both tropical and subtropical production systems. Global eggplant production reached about 55 million tons in 2020, reflecting its wide adaptation and strong market demand, while its continued importance in Asia and the Mediterranean has made it a major target for both productivity improvement and sustainable intensification efforts (Kappel et al., 2024). Despite this importance, eggplant productivity remains uneven across regions because production is constrained by a combination of biotic, abiotic, and management-related factors. Low yields are linked to pest pressure, soil-borne and foliar diseases, temperature and water stress, and inadequate agronomic practices, while many cultivated genotypes still lack sufficient resistance to these stresses under field conditions. These constraints are especially serious in intensive and continuous cultivation systems, where repeated cropping increases inoculum pressure and accelerates soil fatigue. In such settings, bacterial wilt and fungal diseases are among the most damaging constraints, with fungal pathogens alone causing severe economic losses and bacterial wilt frequently producing devastating stand losses in long-term production areas. Conventional approaches based on chemicals, biological agents, or host resistance have often provided incomplete control, particularly for persistent soil-borne pathogens. This production context creates a strong need for management strategies that stabilize yield, reduce crop vulnerability, and remain feasible under commercial field and protected-cropping conditions (Sivasankarreddy et al., 2024).
Within this context, grafting has become an important sustainable technology in vegetable production because it combines a desirable scion with a rootstock selected for stress tolerance, disease resistance, and vigorous root performance. It is now widely regarded as one of the most valuable tools available against soil-borne diseases and adverse environments, and its expansion accelerated after restrictions on environmentally harmful soil fumigants increased the need for non-chemical alternatives in intensive vegetable systems (Tsaballa et al., 2021). The agronomic value of grafting extends beyond disease control. Reviews across vegetable crops show that grafting can increase yield, improve tolerance to drought, salinity, temperature extremes, waterlogging, nematodes, and other biotic or abiotic stresses, while also supporting longer production cycles and lower dependence on agrochemicals (Kappel et al., 2024). In eggplant, these benefits are particularly relevant because the crop is frequently cultivated in soils affected by wilt complexes and in environments where water scarcity or climatic instability limits productivity. Rootstocks can improve water and nutrient uptake, strengthen plant vigor, and buffer the scion against stress through changes in root architecture, xylem transport, antioxidant activity, and hormonal signaling (Musa et al., 2020). Grafting is therefore not simply a rescue technique for diseased fields; it is increasingly viewed as part of a broader low-input and climate-resilient production strategy. At the same time, its practical value depends on rootstock-scion compatibility, nursery skill, and the ability to offset higher transplant cost through gains in yield, quality, and crop reliability (Awazade and Verma, 2024).
Research on eggplant grafting has expanded from simple compatibility testing to a broader analysis of how rootstocks influence growth, physiology, yield, fruit quality, and adaptation to stress. Early and ongoing work has shown that eggplant benefits substantially from grafting and that a wide range of rootstocks, including Solanum torvum, S. macrocarpon, S. aethiopicum, allied species, and interspecific hybrids, can improve vigor and productivity while offering alternatives where rootstock rotation or local adaptation is needed. Experimental studies consistently report higher total or marketable yield in grafted plants than in self-rooted controls, although the magnitude of improvement depends strongly on the specific graft combination. For example, grafting onto wild relative rootstocks increased vigor and marketable yield in multiple scion backgrounds, and some combinations based on S. torvum or S. aethiopicum increased marketable yield by about 20%~31% relative to non-grafted plants (Musa et al., 2020). More recent work has also clarified some of the mechanisms underlying these responses. Rootstocks with stronger root systems and favorable anatomical traits, such as wider xylem or greater root volume, are associated with better water and nutrient acquisition, improved photosynthetic performance, and higher fruit yield, indicating that grafting effects on production are mediated through whole-plant physiological integration rather than simple disease escape alone (Kappel et al., 2024). Even so, the literature also shows that responses in fruit quality traits are less uniform, with some traits improving, some remaining unchanged, and others varying by environment, harvest maturity, and rootstock-scion interaction.
Current eggplant grafting research increasingly emphasizes performance under specific stress scenarios and integrated production systems, which makes the subject especially relevant for a study focused on growth and yield. Under deficit irrigation, grafted eggplant has shown clear advantages over non-grafted plants through stronger canopy vigor, greater root proliferation, improved water and nutrient uptake, and better maintenance of fruit yield and water productivity; in one recent field study, grafting improved fruit yield by 12.7%-24.5% and reduced yield losses under water deficit while maintaining key fruit-quality traits (Wakchaure et al., 2025). Likewise, under semi-arid conditions, drought-tolerant wild rootstocks such as S. sisymbriifolium and S. torvum outperformed non-grafted plants under both full and deficit irrigation, indicating that rootstock choice can materially alter growth and yield stability when water is limiting (Khapte et al., 2025). Beyond water stress, grafting can also reshape the rhizosphere environment, as grafted eggplants have shown increased microbial biomass, greater enzyme activity, lower bacterial wilt incidence, and higher yield than non-grafted controls, suggesting that soil biological effects may contribute to plant performance. Against this background, the objective of the present paper is to examine the effects of grafting on the growth and yield of eggplant, with particular attention to how grafting modifies vegetative vigor, physiological performance, and productivity through rootstock-mediated mechanisms under practical production conditions (Tsaballa et al., 2021).
2 Principles and Mechanisms of Eggplant Grafting
2.1 Graft compatibility and formation of vascular connections
Graft compatibility in eggplant depends on whether the scion and rootstock can heal into a single mechanically stable plant with continuous nonvascular and vascular connections, rather than merely surviving after grafting. Within Solanaceae, compatibility is often strongest in closely related combinations, and tomato-eggplant unions are a clear example of successful intrageneric heterografts in which substantial vascular reconnection supports long-term stability. The graft union forms through a sequence of wound healing events that includes tissue adhesion, vigorous callus proliferation, and later differentiation of new xylem and phloem across the interface (Habibi et al., 2022). During this process, phloem typically reconnects before xylem, and cell-to-cell communication is established through newly formed plasmodesmata, allowing the two partners to coordinate regeneration before the vascular system is fully restored (Tsaballa et al., 2021).
Compatibility is also expressed anatomically at the graft junction. In eggplant-related systems, a successful union is associated with degradation of necrotic layers, close linkage of callus cells, and strong integration between the callus bridge and the vascular network, whereas persistent mismatch at the junction signals functional imbalance (Kappel et al., 2024). Practical assessments therefore often use affinity indices based on the relative diameters of the graft partners, because a balanced junction is more likely to support effective transport of water and nutrients through the developing vascular system (Argento et al., 2023). Incompatibility can be immediate or delayed, and delayed incompatibility is especially important because plants may survive for weeks or longer before mechanical weakness and transport failure become obvious. Molecular work indicates that incompatible unions show disrupted vascular strand reconnection and perturbed expression of key vasculature-related genes, while successful union formation depends on regulators such as SlWOX4 and cell-wall remodeling genes including XTH family genes that sustain callus growth and xylem bridge formation.
2.2 Rootstock characteristics and their functional roles
Rootstock choice is central to eggplant grafting because the rootstock largely determines the belowground capacity for water capture, nutrient uptake, stress tolerance, and resistance to soil-borne pathogens (Musa et al., 2020). In practice, wild Solanum rootstocks and selected tomato hybrids are widely used because they can confer higher vigor, stronger root systems, and greater resilience than self-rooted plants. Anatomical traits of the rootstock are one major basis of these functional effects. In grafted eggplant, rootstocks with larger xylem widths and higher cortex cell numbers were associated with higher yield, while Solanum rootstocks also showed larger root volume or xylem area than self-rooted plants or some commercial tomato rootstocks (Kappel et al., 2024). These findings indicate that rootstock-mediated differences in sap flow and tissue organization help regulate the later performance of the scion by shaping transport efficiency from the seedling stage onward.
The functional role of the rootstock becomes especially clear under stress. Under deficit irrigation, grafted eggplants developed greater canopy vigor, root proliferation, water and nutrient uptake, and photosynthetic capacity than non-grafted controls, which translated into lower yield loss and higher water productivity (Wakchaure et al., 2025). This supports the broader view that rootstocks do not simply anchor the plant, but actively regulate scion growth, flowering, fruit set, and stress resistance through whole-plant integration (Liu et al., 2025). Rootstocks also contribute indirectly by modifying the rhizosphere environment and disease pressure. In eggplant, grafting onto superior rootstocks reduced bacterial wilt incidence sharply and increased microbial biomass, enzyme activity, and microbial diversity in the rhizosphere, indicating that rootstock effects extend beyond plant anatomy into soil ecological function (Du et al., 2024). This is agronomically important because eggplant is highly vulnerable to persistent soil-borne pathogens, and resistant rootstocks such as Solanum torvum are already recognized as effective tools for wilt management where other control methods are unreliable (Sivasankarreddy et al., 2024).
2.3 Physiological and molecular responses induced by grafting
Grafting induces broad physiological changes in eggplant by altering water relations, mineral acquisition, chlorophyll status, and overall vigor through the interaction of the scion with a distinct root system (Musa et al., 2020). In experimental eggplant systems, grafted plants often show increased stem diameter, higher chlorophyll values, and higher yield than self-rooted plants, indicating that the physiological response is expressed in both vegetative growth and reproductive performance (Du et al., 2024). These physiological changes are coordinated by long-distance signaling between the graft partners. Evidence across grafted vegetables shows that hormones, minerals, mRNAs, non-coding RNAs, and proteins move through the vascular system and contribute to the regulation of scion phenotype after grafting. Hormonal control is especially important at the union, where auxin, cytokinin, ethylene, gibberellin, and jasmonic acid help coordinate wound healing, vascular differentiation, and rootstock-scion communication (Habibi et al., 2022).
At the molecular level, grafting triggers substantial transcriptional reprogramming, and compatible versus incompatible unions can differ sharply in gene expression patterns. Heterografts tend to show stronger activation of oxidative stress and stress-response genes, whereas successful unions more effectively upregulate genes involved in cell-wall synthesis, wound responses, hormone signaling, and vascular regeneration. This helps explain why graft healing is not only an anatomical process but also a genetically regulated response shaped by recognition, metabolic balance, and signaling across the junction. Eggplant studies further suggest that some graft-induced responses involve epigenetic regulation. Heterografting-associated vigor in eggplant has been linked to genome-wide CHH hypomethylation and altered scion gene expression, supporting the idea that rootstocks can reshape scion phenotype partly through methylation-dependent regulation. More broadly, grafting can induce DNA methylation changes, small-RNA-mediated signaling, and transcriptional reprogramming across the union, making epigenetic control a plausible mechanism by which grafting influences growth, stress responses, and yield-related traits in eggplant.
3 Effects of Grafting on Eggplant Vegetative Growth
3.1 Influence on plant morphological development
Grafting generally enhances vegetative vigor in eggplant, especially when vigorous or wild rootstocks are used. Field evidence showed significant differences between grafted and non-grafted plants in plant height, total leaf area, stem diameter, and chlorophyll index, with the Pala/Köksal F1 combination reaching about 1.0 m in height, 5645.04 cm²/plant leaf area, and a SPAD value of 47.48 (Ulaş, 2021). Greenhouse results similarly found that grafted plants had thicker stems and higher chlorophyll content than self-rooted controls, indicating that grafting promotes stronger shoot development early in crop establishment (Du et al., 2024). The magnitude of morphological improvement depends on the rootstock-scion combination. Grafting onto Solanum torvum or S. aethiopicum increased plant height at 50 days after transplanting by 11.6% and 9%, respectively, relative to non-grafted plants, while combinations involving wild relatives in open-field trials also showed superior overall growth performance across years (Consentino et al., 2022). Not all vigorous combinations are equally desirable, however, because some highly stimulating rootstocks can induce excessive vegetative growth and disorder, as seen in the Beaufort/Black Bell combination, where vegetative traits were highest but compatibility was weaker and growth became imbalanced (Argento et al., 2023).
3.2 Effects on root system development and nutrient uptake
One of the clearest effects of grafting on vegetative growth is the strengthening of the root system. In grafted eggplant, rootstocks significantly increased shoot and root fresh and dry biomass, with Topan/Köksal F1 reaching 66.29 g/plant root fresh weight and 11.05 g/plant root dry weight, well above the non-grafted control (Ulaş, 2021). Similar evidence from low-cost polyhouse production showed that all grafted plants had superior rooting, and the greatest root number, root length, root fresh weight, and root dry weight were recorded with S. torvum, followed by S. khasianum.
These root improvements translate into stronger nutrient acquisition and greater tolerance to low-input or stressful conditions. In a soilless system, plants grafted onto S. torvum had greater plant dry weight and yield than self-grafted controls, and this vigor was directly linked to major root development and higher accumulation of most analyzed mineral ions. More recent work under deficit irrigation likewise found that grafted plants developed greater root proliferation and improved water and nutrient uptake, which helped reduce yield losses under water stress and supported more stable vegetative performance (Wakchaure et al., 2025).
3.3 Regulation of photosynthetic performance and biomass accumulation
Grafting also regulates vegetative growth by sustaining leaf physiology and photosynthetic function. Under salt stress, grafted plants maintained higher photosynthetic pigment levels than non-grafted plants, and both S. grandifolium × S. melongena and S. torvum rootstocks improved chlorophyll fluorescence parameters and reduced Na+ accumulation in the scion, which supported better growth under stress (Mozafarian et al., 2023). Under drought-related stress, grafting combined with vermicompost was positively associated with SPAD, leaf area, relative water content, shoot dry weight, and root fresh weight, indicating coordinated improvement in leaf function and biomass retention (Kıran et al., 2026).
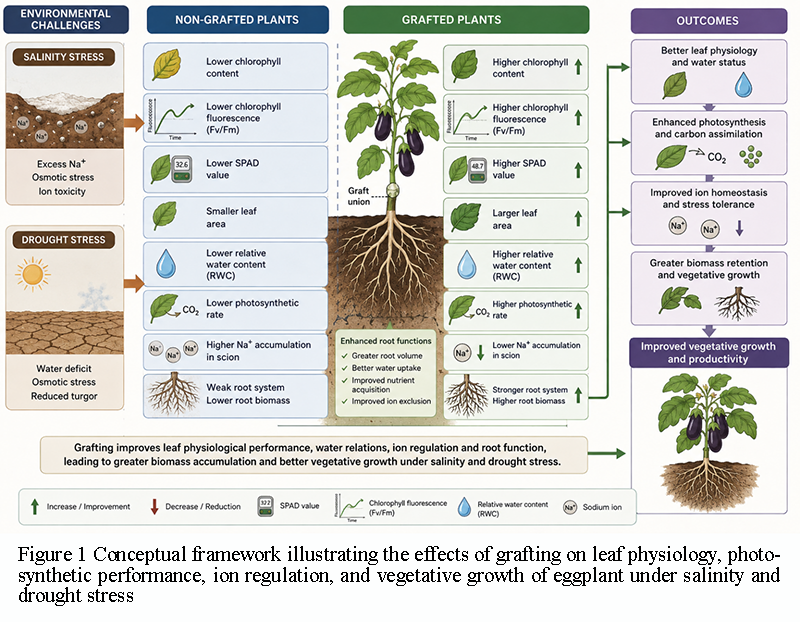
Biomass accumulation in grafted eggplant appears to be driven by improved whole-plant assimilation and allocation rather than by leaf greenness alone. Deficit-irrigation experiments showed that enhanced canopy vigor, photosynthesis, and resource uptake in grafted plants increased fruit yield by 12.7%-24.5% while also supporting shoot biomass under stress (Wakchaure et al., 2025). Anatomical and comparative growth studies further indicate that larger root volume, greater crown diameter, and higher SPAD values are linked with earlier and faster growth in grafted eggplant, while broader grafting research using eggplant rootstocks has associated higher relative growth rate, leaf area ratio, and net assimilation rate with superior grafted-plant performance (Figure 1) (Kappel et al., 2024).
|
Figure 1 Conceptual framework illustrating the effects of grafting on leaf physiology, photosynthetic performance, ion regulation, and vegetative growth of eggplant under salinity and drought stress |
4 Effects of Grafting on Eggplant Yield Formation
4.1 Improvement of flowering and fruit setting characteristics
Grafting can improve reproductive development in eggplant by increasing precocity and supporting earlier transition to effective fruit production when vigorous and compatible rootstocks are used (Musa et al., 2020). In interspecific rootstock systems, the strongest combinations produced greater fruit earliness together with higher early yield, indicating that reproductive advantage begins before final harvest and is closely linked to rootstock vigor and compatibility. This pattern suggests that grafting can shift yield formation forward in time, especially where rapid establishment and strong sink support favor early flowering and fruit retention (Kappel et al., 2024).
The effect on flowering itself is not universally positive, and some studies show that reproductive timing remains highly genotype-dependent. In open-field comparisons, non-grafted CE showed the earliest first flower formation even though several grafted combinations later performed better for overall growth and yield traits (Musa et al., 2020). Reproductive expression after grafting also includes changes in seed set and fruit-setting characteristics, as shown by protected-cultivation work where certain combinations had the highest seed number, confirming that rootstock choice can modify reproductive allocation rather than simply increase vegetative vigor (Mozafarian et al., 2023). Therefore, grafting tends to improve effective fruit setting more consistently than it accelerates first flowering across all scions and environments.
4.2 Effects on fruit yield and yield components
The most consistent effect of grafting on eggplant yield formation is an increase in total and marketable fruit yield, especially when scions are combined with vigorous wild or allied rootstocks. Wild relative rootstocks increased total and marketable yield, fruit number per plant, and average fruit weight relative to non-grafted and self-grafted controls (Musa et al., 2020). Similar results were reported for commercial combinations grafted onto Solanum torvum or S. aethiopicum, where marketable yield increased by 31.4% and 20.0%, respectively, confirming that yield improvement is often expressed through both heavier fruits and more fruits per plant (Consentino et al., 2022).
Yield gains also appear under stress and under protected cultivation, showing that grafting stabilizes productivity rather than acting only in optimal conditions. Under deficit irrigation, grafted plants improved fruit yield by 12.7%-24.5% and reduced yield losses by 12%-44%, while under salinity, grafting onto SH increased total fruit yield mainly through higher average fruit weight (Wakchaure et al., 2025). Greenhouse and field studies likewise found large practical gains, including marketable-yield increases of 53.0% on S. torvum in greenhouse production and total fruit yield of 4711.89 g/plant in the Pala/Köksal F1 combination in the field (Consentino et al., 2022). These responses are commonly attributed to improved water and nutrient uptake from stronger root systems, which increase reproductive support and raise the efficiency of fruit filling (Mauro et al., 2022).
4.3 Effects on fruit quality and nutritional characteristics
Fruit-quality responses to grafting are more variable than yield responses, but favorable combinations often improve commercial and nutritional traits. In one metabolomic and transcriptomic study, the Sm64R rootstock increased fruit size, yield, total soluble solids, phenolic acids, total amino acids, total sugar, and vitamin C, with associated changes in phenylpropanoid, phospholipid, and nucleotide metabolism (Yan et al., 2023). Other studies similarly found that grafting can increase ascorbic acid, chlorogenic acid, protein, potassium, and zinc, while lowering glycoalkaloids, indicating that some rootstocks enhance both nutritive value and functional quality ( Consentino et al., 2022; Sabatino et al., 2022).
At the same time, quality outcomes are not uniform across cultivars, seasons, or rootstocks. Reviews and experiments agree that traits such as soluble solids, peel color, firmness, phenolics, and sensory properties can increase, decrease, or remain unchanged depending on the graft combination and environment. For example, grafting onto S. torvum sometimes reduced total phenolics or altered fruit color negatively, whereas other combinations increased total phenols, calcium, boron, zinc, and overall nutraceutical composition under more targeted nutrient management (Mauro et al., 2022). Overall, grafting improves eggplant yield formation most reliably through higher fruit number, fruit weight, and marketable yield, while fruit quality enhancement depends on selecting rootstocks that match the scion, environment, and production objective.
5 Role of Grafting in Enhancing Stress Resistance of Eggplant
5.1 Resistance to soil-borne diseases and pathogens
Grafting has become a central strategy for protecting eggplant against soil-borne pathogens because susceptible scions can be combined with rootstocks that express broader resistance than cultivated eggplant alone (Musa et al., 2020). This role is especially important in intensive production systems, where continuous cropping increases inoculum pressure and severe yield losses from bacterial wilt, Fusarium wilt, Verticillium wilt, nematodes, and related root diseases can accumulate rapidly (Akanksha et al., 2025). In practical terms, grafting is now used not only to reduce infection in a single crop cycle but also to limit disease development and suppress inoculum build-up in the soil, which improves the health of subsequent crops (Thies, 2021). Experimental evidence in eggplant shows that this protection can be large. In greenhouse production, grafting onto ‘Huimei Zhenba’ reduced bacterial wilt incidence to 3.33% compared with 55.56% in non-grafted controls, while also increasing yield substantially. Under artificial pathogen pressure, grafted plants also showed strong resistance to Verticillium and Fusarium wilts: Hawk and KingKong F1 were completely resistant to Verticillium, and several rootstocks showed complete resistance to Fusarium, with Hawk increasing marketable yield by 68.28% over the non-grafted control under Fusarium stress. Rootstock screening further supports the durability of this approach, with S. torvum showing the strongest multi-pathogen resistance among tested germplasm for bacterial wilt, southern blight, and Fusarium wilt (Akanksha et al., 2025).
Disease suppression by grafting is not explained by host resistance alone, because the rootstock also reshapes the rhizosphere environment in ways that favor plant health. Grafted eggplants had higher microbial biomass carbon, nitrogen, and phosphorus, together with higher phosphatase and β-glucosidase activity, indicating a more active and nutrient-cycling rhizosphere than self-rooted plants. These shifts likely matter biologically because soil microbial communities, biomass, and enzyme activity are recognized determinants of nutrient cycling, soil fertility, and the severity of soil-borne disease expression around the root zone (Du et al., 2024). Even with these clear benefits, resistance remains rootstock-dependent rather than universal. Reviews emphasize that disease-resistant rootstocks are a sustainable replacement for heavily chemical disease management, but they also note the need to expand the rootstock pool because pathogen populations evolve and currently favored resistance sources may not remain sufficient indefinitely (Thies, 2021). Accordingly, future improvement in pathogen resistance will depend on broader rootstock breeding, especially for combinations that retain high compatibility while combining resistance to bacterial wilt, Fusarium, Verticillium, nematodes, and other persistent soil pests (Akanksha et al., 2025).
5.2 Tolerance to abiotic stress conditions
Grafting also improves eggplant tolerance to abiotic stress, particularly drought and salinity, by allowing sensitive commercial scions to exploit the root systems of more tolerant wild or interspecific rootstocks. This is agronomically important because eggplant is drought-sensitive, and water restriction reduces both yield and fruit quality, while salinity creates ionic and osmotic stress that constrains growth and productivity. Across vegetable systems, grafting is therefore treated as a rapid, non-chemical alternative to breeding for resistance to drought, salinity, temperature stress, and related environmental constraints. Under drought, grafted eggplants consistently retain higher productivity than non-grafted plants. In a two-year field study, grafting onto wild rootstocks improved fruit yield by 12.7%-24.5%, reduced yield losses by 12%-44%, and increased water productivity under deficit irrigation through stronger canopy vigor, root proliferation, water uptake, and photosynthesis (Wakchaure et al., 2025). A second semi-arid field study found that SUR/SIS and SUR/TOR outperformed non-grafted Suraj under both full and deficit irrigation, and at 60% ETc the yield reduction was only 14% for SUR/SIS versus 25% for the non-grafted control (Khapte et al., 2025). These responses are consistent with the broader mechanism proposed for grafted vegetables: drought-tolerant rootstocks improve soil exploration, osmotic adjustment, and stress buffering through deeper and more vigorous roots (Nadoda et al., 2024).
Salinity tolerance shows a similarly clear pattern. In eggplant, SH and ST rootstocks protected the scion under 80 mM NaCl by maintaining higher photosynthetic pigment concentration and chlorophyll fluorescence and by lowering Na+ accumulation in the shoot relative to non-grafted plants (Mozafarian et al., 2023). Mechanistically, salinity tolerance depends strongly on ion partitioning, because tolerant rootstocks can retain more Na+ in roots while helping preserve higher K+/Na+ balance and water status in active tissues under saline. The abiotic benefits of grafting extend beyond drought and salinity. Reviews indicate that tolerant rootstocks can also reduce damage from high and low temperatures, flooding, heavy metals, and other adverse soil conditions, although the strength of evidence in eggplant is better for drought and salinity than for all other stresses (Nadoda et al., 2024). Postharvest work also suggests that rootstock-mediated stress protection can persist after harvest, as grafting onto the cold-tolerant ‘Java’ rootstock reduced chilling injury, softening, and pulp browning during cold storage.
5.3 Improvement of resource use efficiency
A third major contribution of grafting is improved resource use efficiency, especially for water and nutrients. This effect is closely tied to the functional role of the rootstock, since vigorous root systems can enhance nutrient uptake, water transport, and osmoregulation under stress while sustaining productive growth (Musa et al., 2020). Root traits are central here: deep and robust roots improve access to soil water and nutrients, and anatomical studies in grafted eggplant show that Solanum rootstocks often produce greater root volume and wider xylem, traits that correlate positively with yield (Kappel et al., 2024). Water use efficiency is one of the best documented outcomes. In a Mediterranean greenhouse, the highest WUE for fruit production occurred in the IR50 treatment with To/Bb, showing that grafting onto S. torvum can convert moderate water limitation into more efficient yield formation rather than simply buffering damage (Argento et al., 2023). Under semi-arid deficit irrigation, SUR/SIS achieved 9.47 kg/m3 water productivity and SUR/TOR 8.22 kg/m3, both above the non-grafted control at 6.72 kg/m3, confirming that rootstock choice can materially improve output per unit water (Khapte et al., 2025). These gains appear to arise from better soil-plant water balance, sustained PSII efficiency, and stronger antioxidative defense under water deficit (Nadoda et al., 2024).
Nutrient use efficiency also improves when grafting enhances root function and rhizosphere activity. Comparative studies report that grafting can increase tissue concentrations or uptake efficiency of major nutrients such as N, P, and K, while greater root activity and xylem development support more effective mineral translocation to the shoot (Yang et al., 2026). In grafted eggplant specifically, enhanced microbial biomass and enzyme activity in the rhizosphere indicate faster nutrient cycling and a more nutrient-rich root environment, which likely contributes to stronger growth and stress resilience (Argento et al., 2023). Resource-use benefits can be strengthened further when grafting is combined with complementary soil management. Integrating grafted plants with vermicompost under moderate drought increased shoot fresh weight by 48.81%, reduced yield loss by 96%, and improved irrigation water productivity by 62.79% in greenhouse conditions. Field and greenhouse evidence from the same research line also shows that the grafting-vermicompost combination improves soil moisture retention, mineral content, and total productivity under drought, making it a promising low-input strategy for climate-resilient eggplant production (Kıran et al., 2026).
6 Case Study: Evaluation of Grafting Effects on Eggplant Growth and Yield under Protected Cultivation
6.1 Experimental design and grafting treatments
Protected-cultivation studies on eggplant grafting generally use comparative designs that include non-grafted and self-grafted controls alongside one or more commercial or wild rootstocks, allowing the specific contribution of the rootstock to be separated from the grafting procedure itself. In unheated greenhouse and tunnel systems, common experimental materials include scions such as ‘Madonna’, ‘Birgah’, or locally adapted cultivars grafted onto Solanum torvum, allied Solanum species, or tomato rootstocks such as Optifort and Emperador (Argento et al., 2023). The cultivation environment is also a defined treatment component in these case studies. Greenhouse experiments have been conducted in soilless pot culture, polyethylene-covered tunnels, unheated plastic houses, and low-cost polyhouses, often with drip irrigation, mulching, and standardized fertigation so that treatment differences mainly reflect graft combination rather than uneven crop management (Sabatino et al., 2022). Some protected-cultivation studies explicitly add environmental or stress factors to the design, such as saline versus non-saline nutrient conditions or heated versus cold greenhouse and substrate regimes, in order to test whether grafting effects remain stable under suboptimal production environments (Mozafarian et al., 2023).
The grafting methods used are usually simple nursery techniques chosen for reproducibility and high survival. Tube grafting, splice grafting, cleft grafting, and clip fixation during healing are all represented in the eggplant literature, followed by a healing and acclimatization period before transplanting into the protected structure. High graft success is repeatedly reported when compatible rootstocks are used, including complete success in some interspecific and wild-rootstock combinations, which supports the feasibility of protected-cultivation trials at commercial scale. Treatment structures also increasingly include integrated inputs intended to test sustainability rather than grafting alone. Recent greenhouse studies combined grafting with arbuscular mycorrhiza, microbial or seaweed-derived biostimulants, or vermicompost so that performance could be evaluated under a broader low-input management framework. This broader design logic is useful for protected cultivation, where growers are interested not only in absolute yield but also in nutrient use efficiency, reduced disease risk, and improved return on intensive infrastructure and input costs (Figure 2) (Sabatino et al., 2022).
|
Figure 2 Experimental framework commonly used in protected-cultivation studies evaluating eggplant grafting performance |

6.2 Effects of different grafting treatments on growth and physiological traits
Across protected systems, different grafting treatments produce clear differences in vegetative growth and physiological status. In greenhouse eggplant, grafted plants commonly show larger stem diameter, higher SPAD values, and greater general vigor than self-rooted controls, and these responses are strongest with vigorous Solanum rootstocks such as S. torvum or selected wild eggplant materials (Sabatino et al., 2022). In seedling and early growth analyses, rootstock effects also extend belowground, with Solanum rootstocks tending to produce larger root volume and wider xylem development, traits that are associated with stronger subsequent growth and better crop performance. Physiological improvement under protected cultivation is closely tied to rootstock-mediated uptake and transport processes. Stronger roots improve water and nutrient acquisition and help maintain chlorophyll status and photosynthetic efficiency, which explains why grafted plants often outperform non-grafted plants even when greenhouse management is otherwise optimized (Kappel et al., 2024). Under salinity in protected soilless culture, grafted plants maintained higher photosynthetic pigment concentrations and chlorophyll fluorescence while retaining more Na+ in roots than in shoots or fruits, indicating that ion partitioning is a major mechanism of physiological protection (Mozafarian et al., 2023).
Not all rootstocks generate equally balanced growth responses. Some combinations stimulate desirable vigor and leaf development, while others induce excessive vegetative growth or functional imbalance, particularly when compatibility is weaker or when the rootstock is too vigorous for the scion (Argento et al., 2023). This makes rootstock selection a physiological decision as much as a disease-management one, because the best protected-cultivation combinations are those that enhance vigor without disrupting reproductive balance or plant architecture (Yan et al., 2022). Protected-cultivation studies also show that grafting can alter the rhizosphere and thereby indirectly affect plant physiology. In greenhouse trials, grafted eggplants had higher microbial biomass carbon, nitrogen, and phosphorus and higher enzyme activity in the rhizosphere, supporting a more active nutrient-cycling environment around the roots (Du et al., 2024). When grafting is combined with beneficial biological inputs such as arbuscular mycorrhiza, these physiological gains can extend to stronger nutrient assimilation and higher nitrogen use efficiency, reinforcing the functional advantage of grafted plants under protected production (Sabatino et al., 2020).
6.3 Effects on yield performance and production sustainability
Yield performance under protected cultivation generally improves when eggplant scions are grafted onto vigorous and compatible rootstocks. In an unheated polyethylene greenhouse, grafting ‘Madonna’ onto S. torvum, SH, or A increased total marketable yield markedly relative to self-rooted plants, with S. torvum reaching 3.94 kg/plant versus 1.65 kg/plant in the control (Mozafarian et al., 2023). Similarly, greenhouse work focused on rhizosphere microecology reported yield increases of up to 36.89% for plants grafted onto ‘Huimei Zhenba’ and substantial gains also for S. torvum, showing that the yield advantage persists across distinct protected-cropping systems (Du et al., 2024). Yield gains are usually expressed through more than one component. Depending on the graft combination, grafted plants can produce more marketable fruits, greater mean fruit weight, or both, and several studies show that the strongest rootstocks improve reproductive output without necessarily compromising apparent fruit quality (Sabatino et al., 2020). In some greenhouse studies, however, quality-related responses are mixed, with certain combinations lowering soluble solids or firmness, which means that higher yield does not automatically translate into better quality across all scion-rootstock pairs.
From a sustainability perspective, protected-cultivation grafting is valuable because it stabilizes production under disease pressure and reduces dependence on chemical soil disinfestation. Grafting emerged partly as a response to restrictions on soil fumigants, and in intensive greenhouse systems it functions as a non-chemical tool to sustain yield where continuous cropping and soil-borne diseases would otherwise reduce plant survival and marketable output (Kappel et al., 2024). This role is reinforced by direct disease outcomes in greenhouse eggplant, where superior rootstocks greatly lowered bacterial wilt incidence while simultaneously increasing yield, making grafting both a protective and productive intervention (Du et al., 2024). Production sustainability under protected cultivation also improves when grafting is integrated with complementary low-input practices. In greenhouse eggplant, combining grafting with microbial biostimulants, mycorrhiza, or vermicompost improved nitrogen use efficiency, marketable yield, and several nutritional traits, suggesting that grafting can serve as the structural platform for broader input-efficient production systems (Sabatino et al., 2020; Consentino et al., 2022).
Even so, the economic value of grafting remains treatment-dependent, because rootstock compatibility, seedling cost, and management complexity still determine whether the biological gains achieved in protected cultivation translate into a consistently scalable production strategy (Argento et al., 2023; Kıran et al., 2026). In protected cultivation, eggplant grafting is most effective when the experimental system uses well-matched rootstock-scion combinations and evaluates both yield and resource efficiency. Across the available case studies, the most reliable outcome is higher and more stable production, especially with Solanum torvum and related vigorous rootstocks.
7 Advances and Future Perspectives of Eggplant Grafting Technology
7.1 Optimization of rootstock selection and grafting methods
Future progress in eggplant grafting depends first on improving rootstock selection beyond the current reliance on a few standard materials. Reviews emphasize that the available rootstock pool remains narrow relative to the diversity of stresses growers face, and that rapid pathogen evolution and complex abiotic-stress traits make it necessary to expand screening and evaluate new rootstock-scion combinations more systematically. This need is reinforced by the strong performance of alternative genetic resources, including interspecific hybrids and wild relatives, which can match or even substitute for Solanum torvum when compatibility and vigor are high. Recent studies show that rootstock optimization should be based not only on disease resistance or survival, but also on anatomical and physiological traits linked to final productivity. In grafted eggplant, larger root volume, wider xylem, and higher cortex cell number were associated with higher yield, indicating that internal rootstock structure can serve as a more informative selection criterion than gross compatibility alone (Kappel et al., 2024). At the same time, practical screening continues to identify robust candidates such as S. torvum, S. sisymbriifolium, and S. incanum for multi-disease resistance, which is directly relevant for breeding next-generation rootstocks with broader adaptation (Akanksha et al., 2025).
Optimization also extends to the grafting process itself, where high success rates depend on both biological compatibility and technical precision. In eggplant relatives, some interspecific hybrids achieved at least 90% germination and 100% graft success, showing that appropriate rootstock genetics can simplify nursery operations as well as improve field performance. Comparable evidence from alternative rootstock programs found high grafting success for selected materials such as SPA and the hybrids Msa 2/2 E7 and 460 CAL, supporting continued diversification of nursery-ready rootstocks (Du et al., 2024). Method optimization is increasingly tied to automation because manual grafting limits scale, uniformity, and labor efficiency. A fully automatic synchronized grafting machine developed for eggplant tray seedlings achieved 700 grafts per hour, about 95% average success, and zero stem damage, indicating that machine-assisted grafting can improve both throughput and seedling quality (Liu et al., 2025). A separate comparison of manual and robotic brinjal grafting likewise found faster healing, about 96.3% success, and about 689.5 grafts per hour in the best robotic treatment with S. torvum, suggesting that future optimization will combine superior rootstocks with precision nursery engineering.
7.2 Integration of grafting with modern agricultural technologies
A major future direction is the integration of grafting with other sustainable crop-management tools rather than using grafting as a stand-alone intervention. Combined strategies are already showing clear benefits in eggplant, particularly when grafted plants are paired with microbial or biological inputs that improve nutrient uptake, stress buffering, and fruit functional quality. This shift matters because plant responses to grafting remain genotype- and environment-dependent, so integrated protocols are needed to stabilize outcomes across production systems (Kıran et al., 2026). Arbuscular mycorrhiza represents one of the clearest examples of productive integration. Under greenhouse conditions, AM fungi increased marketable fruit, fruit number, and nitrogen use efficiency regardless of graft combination, while the B/T and B/P grafts combined with AMF delivered the best overall results for yield traits, mineral profile, and nutritional quality (Sabatino et al., 2020). These findings suggest that future protected-cultivation systems can use grafting as a structural platform onto which beneficial symbionts are added to enhance nutrient acquisition and functional quality.
Biostimulants and organic amendments provide a second integration pathway. In eggplant, Azospirillum brasilense combined with S. torvum or S. aethiopicum rootstocks enhanced growth, yield, nutritional traits, and nitrogen use efficiency, and the authors identified these combinations as useful for plug-plant production systems seeking more sustainable performance (Consentino et al., 2022). More recent drought-management work similarly showed that combining grafted plants with vermicompost improved yield, soil moisture, mineral status, and antioxidant-related quality traits under greenhouse and field stress, supporting integrated low-input strategies for climate-resilient production (Kıran et al., 2026). Digitalization and mechanization are likely to shape the next phase of adoption. Reviews of grafting technology argue that specialized nurseries equipped with advanced seeders, growth chambers, and acclimatization facilities can improve seedling uniformity, while databases, crop models, and mobile tools could help growers choose the most suitable rootstock-scion combinations (Awazade and Verma, 2024). In parallel, grafting-robot reviews conclude that further progress depends on better machine vision, artificial intelligence, and tighter integration between robotics and seedling biotechnology to produce more universal and intelligent systems (Yan et al., 2022).
7.3 Molecular and omics-based understanding of grafting responses
The molecular basis of eggplant grafting is now moving from descriptive physiology toward integrated omics. Reviews highlight that next-generation sequencing has made it possible to examine genomic interactions across the graft junction, including gene exchange, rootstock-scion communication, and large shifts in scion DNA methylation that may underlie graft-induced changes in vigor, stress responses, and quality. This is important because future rootstock selection is unlikely to become truly predictive until molecular markers are connected to agronomic performance. Eggplant-specific evidence already shows that grafting can trigger strong epigenetic reprogramming. Heterografting-induced vigor was associated with genome-wide CHH hypomethylation and altered scion gene expression, linking improved plant performance to epigenetic remodeling rather than to anatomy alone. More broadly, epigenetic diversity is now being considered a usable source of phenotypic variability, with potential value for breeding and for designing graft combinations that are more resilient under changing environments (Tsaballa et al., 2021).
Transcriptomics and metabolomics are also clarifying how grafting alters fruit composition and stress biology. In eggplant, integrated metabolomic and transcriptomic analysis showed that the Sm64R rootstock improved fruit size and several nutritional traits, while differential metabolites and genes clustered in phenylpropanoid, phospholipid, and nucleotide metabolism pathways (Yan et al., 2022). Cold-stress transcriptomics further showed thousands of differentially expressed genes between self- and heterografted combinations, with enrichment in hormone signaling and arginine-proline metabolism, indicating that graft-mediated stress tolerance is regulated through broad transcriptional networks rather than single genes. A further frontier is the study of mobile regulatory molecules as direct mediators of rootstock effects. Under cadmium stress, grafting onto S. torvum reduced fruit Cd by 76% and identified five key differentially expressed miRNAs whose targets were involved in hormone signaling and ion transport, suggesting a mechanistic link between long-distance RNA signaling and safer fruit production (Chenshu et al., 2026). Together with broader evidence that grafting can involve genetic exchange and methylation changes across the union, these findings indicate that future eggplant grafting technology will increasingly rely on omics-guided rootstock design, not just empirical nursery testing (Tsaballa et al., 2021).
8 Conclusions
Across studies, grafting consistently improved eggplant vegetative vigor, root development, and reproductive performance relative to non-grafted controls. Field and greenhouse experiments reported significant increases in plant height, leaf area, chlorophyll status, fruit number, and total yield, showing that rootstocks alter both source strength and sink development rather than only protecting plants from stress. This effect appears strongest when vigorous and compatible rootstocks such as Solanum torvum, wild relatives, or selected interspecific hybrids are used, because these combinations enhance biomass production and support earlier or more sustained fruiting. The yield advantage of grafting is mechanistically linked to stronger root systems, improved water and nutrient uptake, and more stable physiology under stress. Soilless and deficit-irrigation studies showed that vigorous rootstocks increased plant dry weight and yield through greater root development, while also improving water productivity and reducing yield losses under drought. Fruit-quality responses were more variable than growth and yield responses, but several studies still found gains in soluble solids, chlorogenic acid, vitamin C, amino acids, antioxidants, and mineral composition when favorable rootstock-scion combinations were selected.
From a production standpoint, grafting is now a practical tool for stabilizing eggplant performance in intensive and low-input systems. It is especially valuable where continuous cropping and soil-borne diseases limit conventional cultivation, because resistant rootstocks can sharply reduce disease incidence while maintaining or increasing yield under commercial greenhouse conditions. This makes grafting relevant not only for yield improvement, but also for lowering dependence on chemical soil disinfestation and supporting more resilient production systems under protected and open-field cultivation. The technology also has clear value for resource-efficient horticulture. Vigorous rootstocks maintained higher biomass and yield even under reduced nutrient supply, suggesting that fertilizer inputs can be lowered without proportional productivity loss, while other studies documented marked gains in water use efficiency under deficit irrigation. In practice, these benefits can be strengthened further when grafting is combined with complementary approaches such as arbuscular mycorrhiza, microbial biostimulants, or vermicompost, which improved nitrogen use efficiency, fruit nutritional quality, and drought resilience in integrated systems.
Future progress in eggplant grafting depends on moving from empirical rootstock choice to more predictive selection based on compatibility, anatomy, stress tolerance, and target production environment. Current evidence shows that rootstock performance is not universal, and some highly vigorous combinations can cause low compatibility or vegetative imbalance, making it essential to match rootstock and scion more precisely. Root anatomical traits such as xylem width, cortex cell number, and root volume also correlate with later yield, so these characteristics can serve as useful criteria in future breeding and screening programs. A second priority is deeper mechanistic and technological development. Omics studies show that grafting responses in eggplant involve transcriptomic, metabolomic, and epigenetic reprogramming linked to fruit quality and vigor, while nursery engineering studies indicate that automation can raise grafting efficiency and standardize seedling quality at commercial scale. Overall, the most promising application prospect is an integrated grafting system that combines improved rootstock breeding, precision nursery methods, and stress-adapted crop management to support sustainable eggplant production under increasingly constrained environmental conditions.
Acknowledgments
I extend my sincere gratitude to the anonymous reviewers for their valuable and insightful comments, which have greatly strengthened this paper.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Argento S., Treccarichi S., Arena D., Rizzo G.F., and Branca F., 2023, Exploitation of a grafting technique for improving the water use efficiency of eggplant (Solanum melongena L.) grown in a cold greenhouse in Mediterranean climatic conditions, Agronomy, 13(11): 2705.
https://doi.org/10.3390/agronomy13112705
Awazade A.S., and Verma D., 2024, Advancing vegetable grafting: a comprehensive review of techniques, challenges, and the future of automated solutions, Journal of Scientific Research and Reports, 30(11): 517-530.
https://doi.org/10.9734/jsrr/2024/v30i112580
Consentino B.B., Rouphael Y., Ntatsi G., De Pasquale C., Iapichino G., D’Anna F., La Bella S., and Sabatino L., 2022, Agronomic performance and fruit quality in greenhouse grown eggplant are interactively modulated by iodine dosage and grafting, Scientia Horticulturae, 295: 110891.
https://doi.org/10.1016/j.scienta.2022.110891
Du G., Zhu D., He H., Li X., Yang Y., and Qi Z., 2024, The impact of grafting with different rootstocks on eggplant (Solanum melongena L.) growth and its rhizosphere soil microecology, Agronomy, 14(11): 2616.
https://doi.org/10.3390/agronomy14112616
Habibi F., Liu T., Folta K., and Sarkhosh A., 2022, Physiological, biochemical, and molecular aspects of grafting in fruit trees, Horticulture Research, 9: uhac032.
https://doi.org/10.1093/hr/uhac032
Kappel N., Palla B., Challa L., and Mozafarian M., 2024, Rootstock and scion anatomical parameters in grafted eggplant seedlings, influencing growth and fruit production, BMC Plant Biology, 24(1): 1207.
https://doi.org/10.1186/s12870-024-05926-4
Khapte P.S., Chavan L.S., Changan S.S., Wakchaure G.C., Patil R.A., Yadav L.P., Singh T.H., and Reddy K.S., 2025, Synergistic potential of deficit irrigation and grafted eggplant on wild rootstocks for enhanced growth, yield, and water productivity, Applied Water Science, 15(10): 249.
https://doi.org/10.1007/s13201-025-02504-3
Kıran S., Demir Z., Boyacı H.F., Aydınşakir K., Kuşvuran Ş., Zengin S., and Ellialtıoğlu Ş.Ş., 2026, Integrating grafting and vermicompost for the sustainable management of drought in eggplant cultivation, Scientific Reports, 16(1): 8911.
https://doi.org/10.1038/s41598-026-37509-8
Liu Z., Zhou W., Wang F., Li J., Jiang L., Wang G., and Zhang C., 2025, Advanced design and performance evaluation of an automatic synchronized grafting machine for solanum vulgare, Processes, 13(1): 131.
https://doi.org/10.3390/pr13010131
Mauro R.P., Stazi S.R., Distefano M., Giuffrida F., Marabottini R., Sabatino L., Allevato E., Cannata C., Basile F., and Leonardi C., 2022, Yield and compositional profile of eggplant fruits as affected by phosphorus supply, genotype and grafting, Horticulturae, 8(4): 304.
https://doi.org/10.3390/horticulturae8040304
Mozafarian M., Hawrylak-Nowak B., and Kappel N., 2023, Effect of different rootstocks on the salt stress tolerance and fruit quality of grafted eggplants (Solanum melongena L.), Plants, 12(20): 3631.
https://doi.org/10.3390/plants12203631
Musa I., Rafii M.Y., Ahmad K., Ramlee S.I., Hatta M.M.A., Magaji U., Muhammad I., Chukwu S.C., and Sulaiman N.N.M., 2021, Influence of wild relative rootstocks on eggplant growth, yield and fruit physicochemical properties under open field conditions, Agriculture, 11(10): 943.
https://doi.org/10.3390/agriculture11100943
Nadoda N.A., Barot D.C., Baria V.K., and Chaudhari V.M., 2024, Exploitation of grafting for abiotic and biotic stress management in vegetable crops: a review, Advances in Research, 25: 125-131.
https://doi.org/10.9734/air/2024/v25i41089
Sabatino L., Consentino B.B., Ntatsi G., La Bella S., Baldassano S., and Rouphael Y., 2022, Stand-alone or combinatorial effects of grafting and microbial and non-microbial derived compounds on vigour, yield and nutritive and functional quality of greenhouse eggplant, Plants, 11(9): 1175.
https://doi.org/10.3390/plants11091175
Sivasankarreddy K., Joseph J., Pp T., K P., Thayyil P., Mathew D., and Pathrose B., 2024, An insight into bacterial wilt of eggplant—a review, Tropical Plant Pathology, 49(6): 746-764.
https://doi.org/10.1007/s40858-024-00683-z
Thies J.A., 2021, Grafting for managing vegetable crop pests, Pest Management Science, 77(11): 4825-4835.
https://doi.org/10.1002/ps.6512
Tsaballa A., Xanthopoulou A., Madesis P., Tsaftaris A., and Nianiou-Obeidat I., 2021, Vegetable grafting from a molecular point of view: the involvement of epigenetics in rootstock-scion interactions, Frontiers in Plant Science, 11: 621999.
https://doi.org/10.3389/fpls.2020.621999
Ulaş F., 2021, Response of different rootstocks on vegetative growth, fruit and seed yield of eggplant (Solanum melongena L.), Genetika, 53(2): 593-608.
https://doi.org/10.2298/GENSR2102593U
Wakchaure G.C., Kumar D., Kumar S., Gawhale B.J., Meena K., Sawant C.P., Singh D., Paramasivam S., and Minhas P.S., 2025, Grafting wild rootstocks as a climate-resilient strategy to enhance productivity, quality and tolerance in eggplant under variable water stress induced by deficit irrigation, Agricultural Water Management, 314: 109492.
https://doi.org/10.1016/j.agwat.2025.109492
Yan G., Feng M., Lin W., Huang Y., Tong R., and Cheng Y., 2022, Review and prospect for vegetable grafting robot and relevant key technologies, Agriculture, 12(10): 1578.
https://doi.org/10.3390/agriculture12101578
Yang W.J., Tseng H.Y., Pao Y.C., Mendieta A.B.P., and Rho H., 2026, Grafting onto eggplant rootstock improves water status and fruit quality in tomato under deficit irrigation, BMC Plant Biology, 26(1): 526.
https://doi.org/10.1186/s12870-026-08322-2
. HTML
Associated material
. Readers' comments
Other articles by authors
. Wenjing Xu

Related articles
. Eggplant
. Grafting technology
. Rootstock
. Growth performance
. Yield improvement
Tools
. Post a comment